 Ocean Flux
Teaching · food-web nutrient fluxes
Nutrients move through animals as well as through water
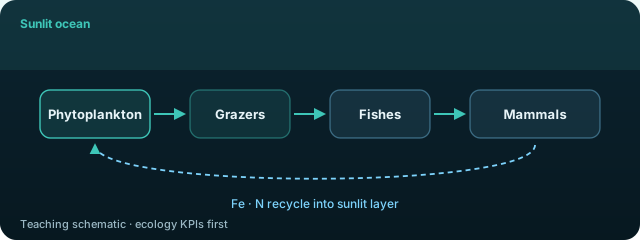
Biological nutrient fluxes run across the food web — not phytoplankton alone. Guilds, grazers, fishes, and marine mammals recycle iron and nitrogen into the sunlit ocean. Ecology KPIs and stop hooks sit above any carbon story.
Ocean Flux framing only · restoration literacy.
Source: Author et al. (Year) = Source tag: the primary source was checked; the tag names it (APA citation, with page or table where we have one) and itself opens the paper (doi.org). Assumption = working hypothesis or teaching value, not a cited source.
Phytoplankton guilds — base of the pump
Functional groups matter more than bulk chlorophyll: picophytoplankton, nanoflagellates, diatoms, dinoflagellates, and diazotrophs such as Trichodesmium.
Guild shifts change export efficiency, silicon demand, toxin risk, and food quality for zooplankton. The explorer’s diatom-fraction slider is a teaching proxy for “export-prone” communities — Assumption teaching proxy pending a surveyed ETP community cite.
Why living cells need iron — enzyme pathways
Iron is not optional flavouring. In ocean microbes it sits inside the proteins that run photosynthesis, turn nitrate into usable nitrogen, and — in nitrogen-fixers — convert N₂ into bioavailable N. Restoring regenerative Fe cycling matters because those pathways fail when bioavailable Fe is scarce. Explorer still reports tonnes C and N; Fe stays a driver.
-
Photosynthetic pathways
Photosynthetic electron transport uses iron in photosystems and in cytochrome / iron–sulfur proteins. Without enough bioavailable Fe, scarce Febio limits / impairs the light reactions that fix carbon into biomass. Source: Twining & Baines (2013) (Twining & Baines 2013).
-
Nitrate reduction
Nitrate and nitrite reductase are iron-dependent enzymes. Phytoplankton growing on nitrate therefore carry a higher iron demand than the same cells using ammonium. Source: Maldonado & Price (1996) (Maldonado & Price 1996).
-
Nitrogenase
Nitrogenase, the enzyme that fixes N₂, is iron-rich. Diazotrophs that fix nitrogen raise cellular iron demand — one reason Fe and N limitation are tightly coupled in parts of the ocean. Source: Twining & Baines (2013) (Twining & Baines 2013). Regional weight of diazotrophs in teaching boxes is Unknown until Phase B — Phase A narrative framing only.
-
Nitrogen fixation may be underestimated
A Holocene nitrogen isotope budget implies that, if the isotopic value of marine fixed nitrogen has not changed, about 280 Tg N per year of sedimentary (seafloor) denitrification is needed to balance sources and sinks. “If such a high rate of denitrification has been sustained throughout the Holocene, it implies that present‐day estimates of marine nitrogen fixation are grossly underestimated.” Source: Brandes & Devol (2002) (Brandes & Devol 2002). Nitrate in the deep ocean (below 2.5 km) has a near-uniform δ¹⁵N of 4.8 ± 0.2‰. Source: Sigman et al. (2000) (Sigman et al. 2000). How large the fixation flux is, and how far it can be restored: Unknown
Chemistry sets how much iron is bioavailable (dissolved Fe + ligands). Biology sets which enzymes that iron must feed. → Chemistry
Macroalgae — ocean afforestation potential
Separate from the diatom export path above. This block is about floating seaweed as a carbon-relevant biomass stream alongside the microalgae export path.
-
Green and golden seaweed tides
Green and golden tides of floating macroalgae have become larger and more frequent along many coasts — a coastal hazard and a large biomass source. Source: Smetacek & Zingone (2013) (Smetacek & Zingone 2013).
-
Ocean afforestation (OAFF)
Open-ocean cultivation of seaweed is termed ocean afforestation. “Open-ocean cultivation of seaweed (macroalgae) biomass, termed ocean afforestation (OAFF), is a nature-based method currently in the planning stage for carbon dioxide removal (CDR) at scales relevant to climate intervention.” Source: Smetacek et al. (2024) (Smetacek et al. 2024, direct). The same comment concludes: “We conclude that farming seaweeds has the potential to become an effective, multipurpose, revenue-generating CDR method.” Source: Smetacek et al. (2024) (Smetacek et al. 2024, direct).
One-sentence frame only: Smetacek’s career iron work treats diatom blooms as the export community when conditions allow; the macroalgae comment is a later, separate line on seaweed farming and does not replace that diatom path.
Seagrass and rooted marine plants
Carbon in biomass plus activity, locked into the seabed below the meadow.
-
Seagrass ecosystems “could store as much as 19.9 Pg organic carbon” worldwide; a more conservative estimate is 4.2–8.4 Pg. Source: Fourqurean et al. (2012) Vegetated coastal habitats contribute “about 50%” of ocean carbon burial. Source: Duarte et al. (2005)
-
Sugars under Posidonia oceanica roots reach concentrations “nearly 80 times higher than previously observed in marine environments”, and a nitrogen-fixing symbiont lives inside its root tissue. Source: Sogin et al. (2022) Source: Mohr et al. (2021)
-
29% of the known seagrass area lost since 1879. Source: Waycott et al. (2009) At one long-term restoration site, burial rates matched natural meadows 18 years after planting. Source: Marbà et al. (2015) 3,612 ha restored on the Virginia coast. Source: Orth et al. (2020)
-
Durable while the meadow stands: “loss of seagrass triggers the erosion of historic carbon deposits.” Source: Marbà et al. (2015) Carbonate burial in seagrass “may correspond to an offset of 30%” of net CO₂ sequestration, mostly supplied from adjacent ecosystems. Source: Saderne et al. (2019) Seaweeds could sequester about 173 Tg C a year (61–268), about 90% via export to the deep sea. Source: Krause-Jensen & Duarte (2016) Pristine baseline for a site: Assumption
“The aim is that these are modelled assumptions and site-specific empirical measurements can be incorporated using magnitude sliders representing uncertainty and variability across natural process controls assumed from scientific literature across parameter, criteria and ecosystem dynamics with respect to chemistry, physics and biology terms. Incorporating empirical terms improves model assumptions.” — Neil Beckwith
Grazers, fishes, and the whale pump
- Zooplankton — Grazing regenerates NH₄⁺, DON, and Fe-binding organics in the mixed layer; fecal pellets contribute to export. Recycling in the sunlit zone and packaging for sinking are both fluxes.
- Fishes — Source: Moreno & Haffa (2014) Moreno & Haffa (2014): marine fish store and recycle substantial Fe; commercial harvest removes Fe from the ocean reservoir and forgoes excretion cycling. Global storage and excretion orders reported in that paper are literature estimates; mass-specific rates in the explorer remain Assumption / synthesised (global totals ≠ local ETP rates).
- Marine mammals / whale pump — Source: Roman et al. (2014) Roman et al. (2014): whales as ecosystem engineers — surface fecal plumes recycle N and Fe after deep feeding; migrations move nutrients across latitudes. Source: Savoca et al. (2021) Savoca et al. (2021): tag-based prey consumption revises mysticete intake upward; Southern Ocean mysticetes recycled on the order of ~1.2×10⁴ t Fe yr⁻¹ pre-whaling versus ~1.2×10³ t Fe yr⁻¹ today (paper estimates). Source: Roman & McCarthy (2010) Roman & McCarthy (2010): marine mammals can enhance surface nitrogen availability by feeding at depth and releasing nutrients near the surface (whale pump). Source: Lavery et al. (2010) Lavery et al. (2010): Southern Ocean sperm whales recycle on the order of tens of tonnes of iron per year to surface waters via feces (published estimate) — literature estimate only; never a Flux Explorer headline.
- Microbial loop & ligands — Bacterial remineralisation and organic exudates contribute Fe-binding ligands. Biology supplies ligand-rich organic matter; chemistry sets bioavailability.
Ocean Flux uses restoration of recycling services as a scientific framing.
Ecology-first KPIs
Carbon optionality only after MRV — these teaching KPIs come first.
-
Primary production quality
Guild mix, not Chl-a alone — avoids the “green water = success” fallacy. Metrics remain Assumption until Phase B protocols.
-
Mesozooplankton
Biomass / size spectrum tracks food-web transfer. Explorer defaults are order-of-magnitude teaching values.
-
Higher-trophic indicators
Forage-fish and predator proxies speak to recycling capacity and fisheries co-benefit ethics.
-
Surface dFe + ligands
Bioavailability with the chemistry page — not bulk Fe alone. Export proxies are teaching only.
Stop hooks — STOP / reassess, never “optimise harder”
Hard teaching interlocks for the page and explorer. Caution bands below are Assumption for teaching, not regulatory criteria.
- STOP HAB risk — toxic-guild / dinoflagellate fraction above a caution band, or Si drawn down while N remains high (Si∶N stress favouring non-diatoms). Teaching trip: diatom fraction < 0.15 and surface nitrate > 5 µM.
- STOP Hypoxia / low O₂ — subsurface O₂ below a caution threshold in the analysis box (physics supplies O₂ context). Teaching trip: subsurface O₂ < 60 µmol kg⁻¹.
- STOP Anomalous bloom without grazers — chlorophyll rise with collapsing zooplankton proxy → food-web failure mode.
- STOP Ligand saturation + scavenging — adding an “Fe narrative” when ligands are saturated does not raise Febio (bridge to chemistry).
Flux Explorer — biology inputs
Six teaching sliders. Excluded: dosing recipes as sources.
| Symbol | Label | Unit | Default | Status |
|---|---|---|---|---|
| Bpre | Pristine higher-trophic biomass density | g wet wt m⁻² | 25 | Assumption / derived productive tropical–upwelling teaching density — not ETP surveys |
| EFe | Mass-specific Fe excretion | µmol Fe g⁻¹ d⁻¹ | 0.025 | Assumption synthesised from Moreno & Haffa (2014) global totals |
| δ | Depletion fraction (recycling capacity lost) | fraction 0–1 | 0.67 | Assumption predatory-guild decline order ~two-thirds (literature-informed) |
| fdiatom | Diatom fraction of phytoplankton biomass | fraction 0–1 | 0.40 | Assumption teaching export-prone guild mix |
| Zmeso | Mesozooplankton biomass index | mg C m⁻³ | 20 | Assumption order-of-magnitude teaching default |
| Rwhale | Relative whale-recycling index vs pre-whaling | fraction 0–1 | 0.10 | Assumption teaching from Savoca et al. (2021) SO Fe recycling ~10× lower today — regional teaching magnitude |
Explore in the Flux Explorer. Pair with chemistry bioavailability and physics supply timing.
Key citations
- Moreno, A. R., & Haffa, A. L. M. (2014). The impact of fish and the commercial marine harvest on the global ocean iron cycle. PLOS ONE, 9(9), e107690. https://doi.org/10.1371/journal.pone.0107690
- Roman, J., et al. (2014). Whales as marine ecosystem engineers. Frontiers in Ecology and the Environment, 12(7), 377–385. https://doi.org/10.1890/130220
- Savoca, M. S., et al. (2021). Baleen whale prey consumption based on high-resolution foraging measurements. Nature, 599, 85–90. https://doi.org/10.1038/s41586-021-03991-5
- Moore, C. M., et al. (2013). Processes and patterns of oceanic nutrient limitation. Nature Geoscience, 6, 701–710. https://doi.org/10.1038/ngeo1765
- Twining, B. S., & Baines, S. B. (2013). The trace metal composition of marine phytoplankton. Annual Review of Marine Science, 5, 191–215. https://doi.org/10.1146/annurev-marine-121211-172322
- Maldonado, M. T., & Price, N. M. (1996). Influence of N substrate on Fe requirements of marine centric diatoms. Marine Ecology Progress Series, 141, 161–172. https://doi.org/10.3354/meps141161
- Tagliabue, A., et al. (2017). The integral role of iron in ocean biogeochemistry. Nature, 543, 51–59. https://doi.org/10.1038/nature21058
- Brandes, J. A., & Devol, A. H. (2002). A global marine-fixed nitrogen isotopic budget: Implications for Holocene nitrogen cycling. Global Biogeochemical Cycles, 16(4). https://doi.org/10.1029/2001GB001856
- Sigman, D. M., et al. (2000). The δ15N of nitrate in the Southern Ocean: Nitrogen cycling and circulation in the ocean interior. Journal of Geophysical Research: Oceans, 105(C8), 19599–19614. https://doi.org/10.1029/2000JC000265
Disclaimer strip
Teaching model. Ecology KPIs first. No field dosing. See Disclaimer and Support.